In the early 20th century, British physiologist Archibald Hill studied how muscles contract and noticed a strange pattern: oxygen binding by hemoglobin was not linear but accelerated. He derived an equation that later took root in enzyme kinetics. The essence is simple: many enzyme proteins do not work alone but as a team. When one substrate molecule binds to an enzyme, it facilitates the binding of the next—this is cooperativity. The graph of rate versus concentration resembles an S-shape: a gentle start, a steep rise, a plateau. The Hill equation compresses this behavior into two numbers: the maximum rate and the half-saturation constant—the concentration at which the enzyme is half-loaded. And the cooperativity coefficient (symbol n) tells how cooperatively the subunits work: if n=1, each acts independently; if n>1, it's a chain reaction of mutual help.
History
Archibald Hill, in 1910, while a student at Cambridge, investigated the oxygen dissociation curve for hemoglobin. He noticed that simple hyperbolic models did not describe the S-shaped curve and proposed an empirical equation with a variable exponent. Later, in the 1920s, Leonor Michaelis and Maud Menten developed a more rigorous kinetic theory for non-cooperative enzymes, but the Hill equation remained a convenient tool for rapid assessment of cooperativity. Hill himself received the Nobel Prize in 1922 for his research on muscles, and his equation became a standard in biochemistry and pharmacology.
How it works
It is used to determine binding parameters: from a plot of log(v/(V_max-v)) versus log[S] (Hill plot), the slope of the line gives n, and the intercept gives log(K_0.5). In pharmacokinetics, the equation describes the saturation of drug-metabolizing enzymes, which is critical for dose calculation. Limitations: the model assumes infinite cooperativity (all or nothing), which is rarely realized in real systems; for accurate description of partial cooperativity, models such as Adair-Klotz or Monod-Wyman-Changeux are used.
In practice
Calculating drug doses so that liver enzymes are not overwhelmed by overload, and designing bioreactors with optimal reaction rates.
Fun fact
Hemoglobin is a classic example of cooperativity: in the lungs, it avidly grabs oxygen (n≈2.8), and in tissues, where oxygen is scarce, it just as abruptly releases it. Without this S-shaped curve, we would suffocate even under light exertion.
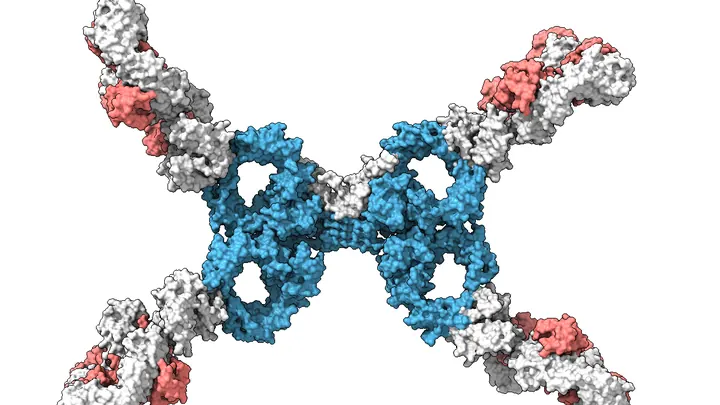
When an antibody meets a virus, it doesn't latch on with a single death grip. Rather, it's like two bunches of grapes tumbling in water, catching each other with dozens of short tendrils. Each tendril is weak on its own, easily torn by the thermal jitter of water molecules, but together they hold tight.
Inside every cell, things are constantly meeting and parting. Some pairs hold tight, like Velcro, while others barely touch, like pollen on the wind. These fleeting touches, where the binding strength is comparable to a grain of salt dissolving in a glass of water, govern many of the cell's signals and decisions.
A choir where every singer hits the notes precisely sounds louder than you'd expect from a simple sum of voices. A hundred singers aren't just a hundred times louder than one: they're ten thousand times louder. In the world of atoms, something similar happens. In collective behavior discovered by Robert H.
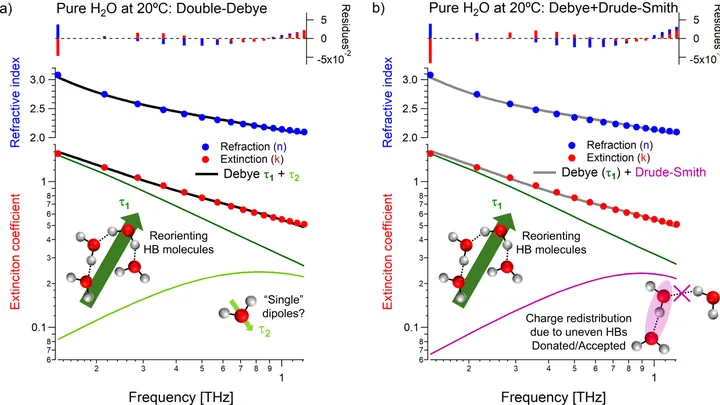
Water is not just a wet substance. On a picosecond scale, it resembles a dance floor where molecules continuously break and form bonds with each other. Usually, this dance is described by one main movement — collective relaxation, as if the whole crowd simultaneously slows down after the music stops.
A kitchen sponge soaked in syrup: in some spots there's more syrup, and your finger sticks right away; in others, it barely touches. That's roughly how a catalyst surface works. Molecules don't react everywhere but at especially sticky points — active sites.
A protein is a tiny magnet with a complex shape, and a nanoparticle is a smooth ball. Depending on which side of the protein approaches the ball, the attraction differs. Scientists have built a detailed map of these "landings" to understand how allergen molecules from birch pollen attach to silica nanoparticles.
They used two approaches.
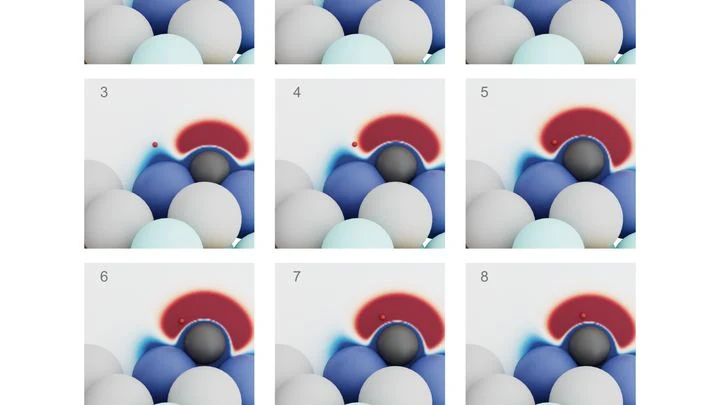
Hydrogen is the lightest fuel, and its conversion into electricity on a metal surface resembles a game of ping-pong: hydrogen atoms alternately attach to and detach from the electrode. But the score in this game depends on solution acidity in ways that were unexpected. Classical formulas predict a smooth change, while experiments show jumps and kinks.
Inside every muscle is a team of rowers: myosin proteins that grab actin filaments, take a stroke, and let go. The fuel for the stroke is the ATP molecule. When the rowers work in sync, the muscle contracts and the body moves.
For decades, two models existed: one explained why the boat moves slower with increasing load, the other — how the rowers move their arms.
An ordinary chemical reaction is like a ball rolling down a hill: it has one natural path. But if you place molecules in a tiny mirrored box, an optical microresonator, the light inside starts to interfere with the ball's motion. It can nudge it, hold it back, or even split its trajectory.
In a new study, physicists traced exactly how this happens.
A translator gets distracted by every rustle in the hall, and a one-hour meeting stretches into two. Single molecules squeezed between two metal contacts behave much the same way: they constantly change their shape and seating, and this affects how current and heat pass through them.
In 1979, Su, Schrieffer, and Heeger proposed a model that explained the strange electrical properties of polyacetylene, an organic polymer that conducts electricity almost like a metal. Their chain consisted of carbon atoms connected alternately by single and double bonds.